By the time a cell has completed the Citric Acid Cycle, it has successfully stripped the original glucose molecule of its high-energy electrons. While the cycle produces a small amount of immediate energy in the form of ATP, its most significant contribution is the "charging up" of specialized molecules called electron carriers. These carriers, NADH and FADH2, act as mobile batteries, transporting high-energy electrons to the inner mitochondrial membrane to fuel the final, most productive stage of cellular respiration: oxidative phosphorylation.
The Goal: Glucose Oxidation and Energy Transformation
To understand the Electron Transport Chain (ETC), we must first look at the big picture of cellular respiration. The overall goal is to take the chemical bond energy stored in glucose and convert it into a form the cell can use: ATP.
The complete oxidation of glucose can be summarized by the following chemical equation:
C6H12O6+6O2ΔG→6CO2+6H2O=−686 kcal/mol
This process is a masterclass in energy transformation. According to the laws of thermodynamics, energy cannot be created or destroyed, only transformed. In the context of the ETC, we see a sequence of energy shifts:
Chemical Bond Energy: Stored in the bonds of glucose and later in the reduced forms of NADH and FADH2.
Positional Potential Energy: Created when electrons drive the pumping of protons ($H^+$) across a membrane, establishing an electrochemical gradient.
Mechanical Kinetic Energy: The flow of protons back through the enzyme ATP synthase causes it to rotate, physically driving the synthesis of ATP.
This diagram illustrates the process of cellular respiration, starting with glucose, moving through the electron transport chain, and resulting in a proton gradient that stores potential energy.
The Players: Electron Donors and Acceptors
The ETC functions like a "daisy chain" of redox reactions. In any redox reaction, one molecule loses electrons (oxidation) while another gains them (reduction).
The Donors: NADH and FADH2
These are our primary electron donors. They arrive from the Citric Acid Cycle carrying high-energy electrons.
NADH: A very powerful carrier. When it is oxidized back to NAD+, it releases a significant amount of free energy.
FADH2: A slightly less powerful carrier than NADH. Because it enters the chain at a later stage, it contributes less to the overall proton gradient.
The Acceptor: Oxygen
For the chain to keep moving, the electrons must have a place to go. Oxygen (O2) serves as the final electron acceptor. At the end of the chain, oxygen picks up the spent electrons along with protons from the surrounding medium to form water (H2O). Without oxygen, the entire chain backs up, and ATP production via this method grinds to a halt.
The Mechanism: The Electron Transport Chain
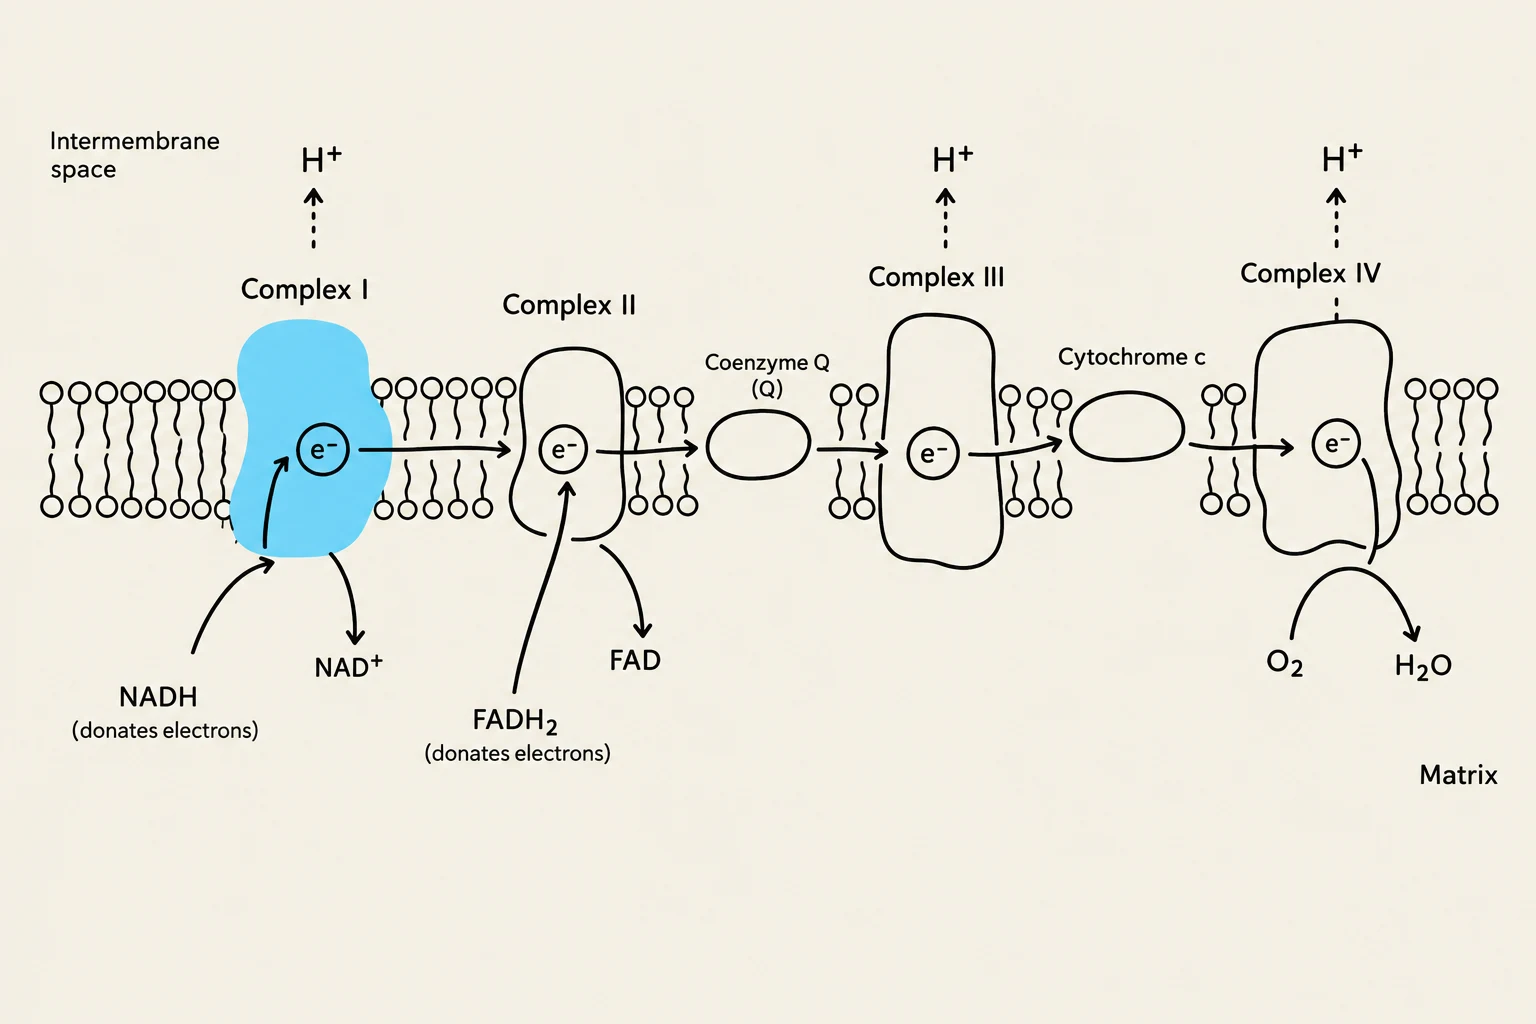
The ETC is composed of four major protein complexes embedded in the inner mitochondrial membrane, along with mobile coenzymes that shuttle electrons between them.
Complex I & II: These are the entry points. NADH delivers its electrons to Complex I, while FADH2 delivers its electrons to Complex II.
Coenzyme Q (Ubiquinone): A mobile, hydrophobic molecule that diffuses through the fatty acid core of the membrane to carry electrons from Complexes I and II to Complex III.
Cytochrome c: A small protein that acts as a shuttle between Complex III and Complex IV.
Complex III & IV: As electrons pass through these complexes, the energy released is used to perform primary active transport.
Exam Tip: Primary Active Transport
Remember that the ETC uses the energy from electron flow to pump protons ($H^+$) across the inner membrane. This is called primary active transport because the energy comes directly from the redox reactions of the electron carriers, not from the hydrolysis of ATP.
Diagram illustrating the electron transport chain in cellular respiration, showing the movement of electrons through protein complexes embedded in the inner mitochondrial membrane, proton pumping, and the final reduction of oxygen to water.
The Proton-Motive Force and ATP Synthesis
As electrons move through the complexes toward oxygen, the energy released is used to pump protons from the mitochondrial matrix into the intermembrane space. This creates a massive concentration imbalance known as the proton-motive force.
This force represents positional potential energy. The protons "want" to flow back into the matrix to reach equilibrium, but the membrane is impermeable to them. They can only pass through a special protein channel called ATP synthase.
As protons rush through ATP synthase, they trigger a physical rotation in the enzyme. This conversion of potential energy into mechanical kinetic energy allows the enzyme to catalyze the phosphorylation of ADP into ATP. This specific process—using the energy of a proton gradient to make ATP—is called oxidative phosphorylation.
Diagram illustrating ATP synthase, a protein complex embedded in the inner mitochondrial membrane, which synthesizes ATP from ADP and inorganic phosphate using the energy from a proton gradient.
Summary Table: Energy Carriers in the Citric Acid Cycle
To prepare for exams, remember how the energy from the previous stages is distributed before it even reaches the ETC:
Molecule
Role in ETC
Energy Potential
NADH
Primary Electron Donor
High
FADH2
Secondary Electron Donor
Moderate
Oxygen (O2)
Final Electron Acceptor
N/A (Forms H2O)
ATP
Final Energy Product
High (Chemical Bond)
Key Concept Check
Why can't we just harvest energy directly from NADH? Because the energy is released in small, discrete steps through the ETC. This allows the cell to use that energy to build a proton gradient incrementally, rather than releasing it all at once as unusable heat.
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.