Prokaryotic Transcription Mechanisms and Regulation
An in-depth explanation of prokaryotic transcription, covering RNA polymerase function, initiation, elongation, termination, and the regulation of gene expression through operons like the Lac operon.
Transcription is the fundamental biological process of transferring genetic information from a DNA template to a mobile RNA molecule. In prokaryotes like E. coli, this process is the first step of the central dogma, allowing the cell to convert the "locked" instructions in the genome into messenger RNA (mRNA), transfer RNA (tRNA), or ribosomal RNA (rRNA). Unlike DNA replication, which copies the entire chromosome, transcription only copies selected fragments of the DNA.
The Machinery of Transcription: RNA Polymerase
The primary engine of transcription is RNA polymerase (RNA pol). In E. coli, this is a large molecule with a molecular weight of approximately $390,000$ Da. The enzyme exists in two functional forms: the core enzyme and the holoenzyme.
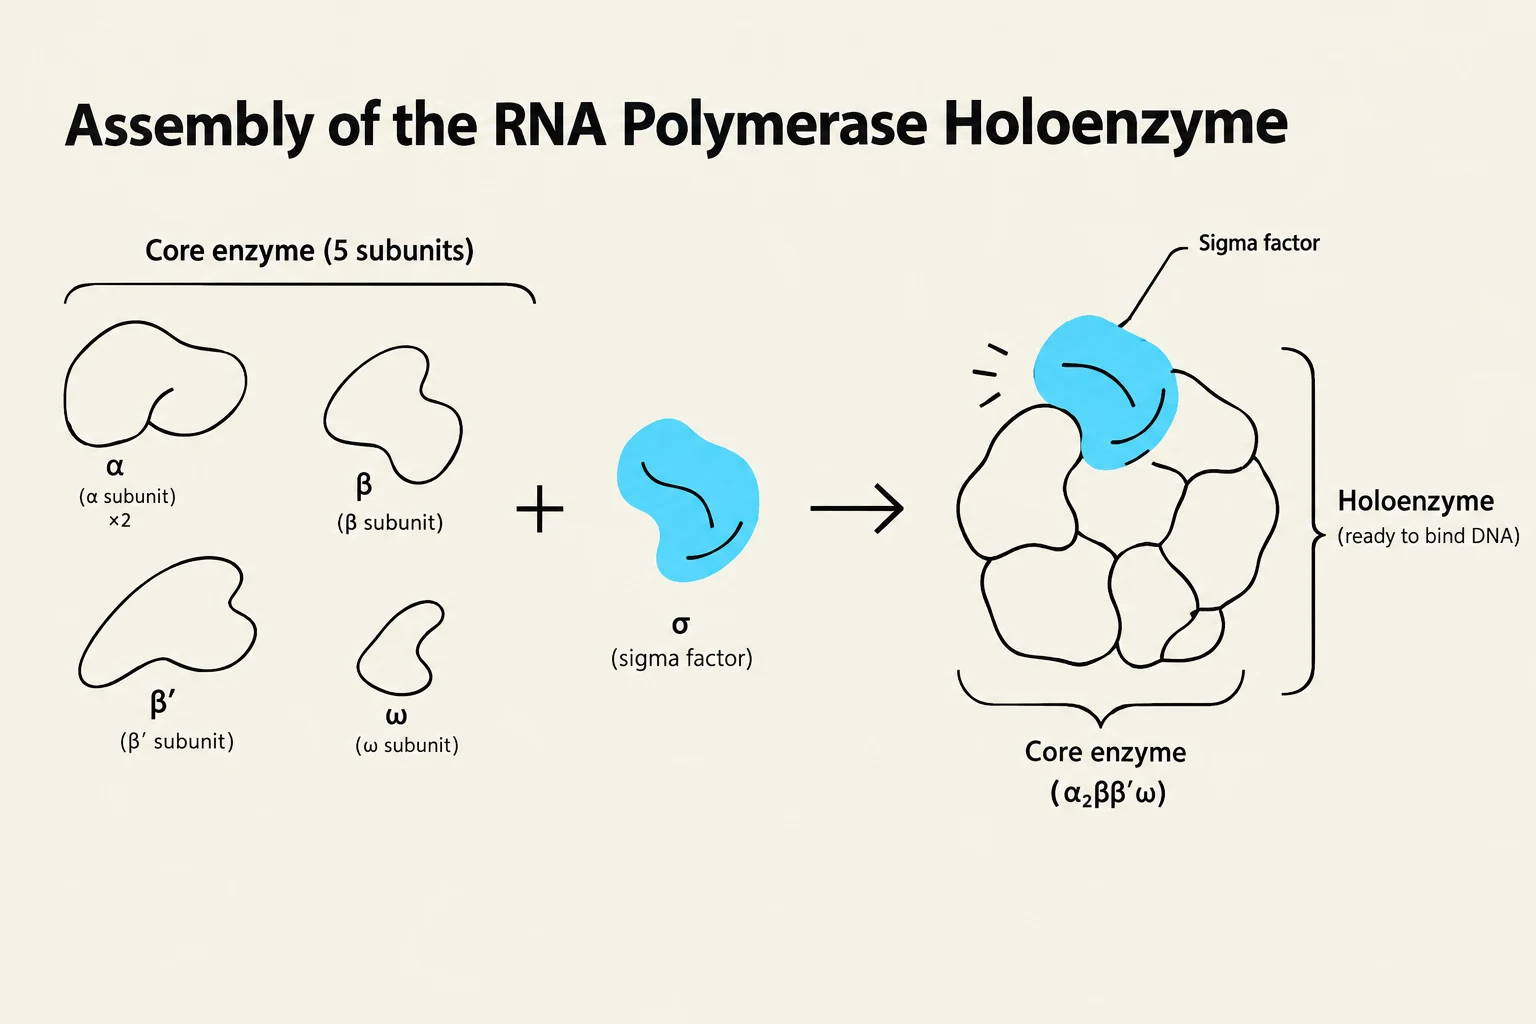
The core enzyme is composed of five subunits (2α, 2β, and ω). While the core enzyme is capable of synthesizing RNA, it lacks the ability to recognize specific starting points on the DNA; without assistance, it has a general affinity for almost any DNA binding site. To achieve specificity, the core enzyme must associate with a sixth subunit called the sigma factor (σ). This association creates the functional holoenzyme, which is capable of precisely locating and binding to specific promoter sequences.
Exam Tip: Remember that the core enzyme performs the actual polymerization, but the sigma factor is the "GPS" that provides promoter specificity.
Diagram illustrating the assembly of the RNA Polymerase Holoenzyme, showing the combination of the core enzyme (composed of alpha, beta, beta-prime, and omega subunits) with the sigma factor to form the holoenzyme, which is ready to bind DNA.
Initiation: Finding the Start
Transcription begins at specific DNA sequences known as promoters. These regions direct the start of transcription and are typically located between −70 and +30 relative to the transcription start site (where the first nucleotide of the RNA is designated as +1).
Promoter Architecture
Key regulatory elements within the promoter include:
The −10 and −35 regions: These are critical sequences that the RNA polymerase recognizes to ensure it binds at the correct location.
The UP element: Located further upstream between −60 and −40, this element binds to the α subunit of the RNA polymerase, significantly enhancing high levels of gene expression.
The Initiation Sequence
Once the holoenzyme identifies the promoter, the process moves through several distinct stages:
Closed Complex: The RNA polymerase binds to the promoter while the DNA remains double-stranded.
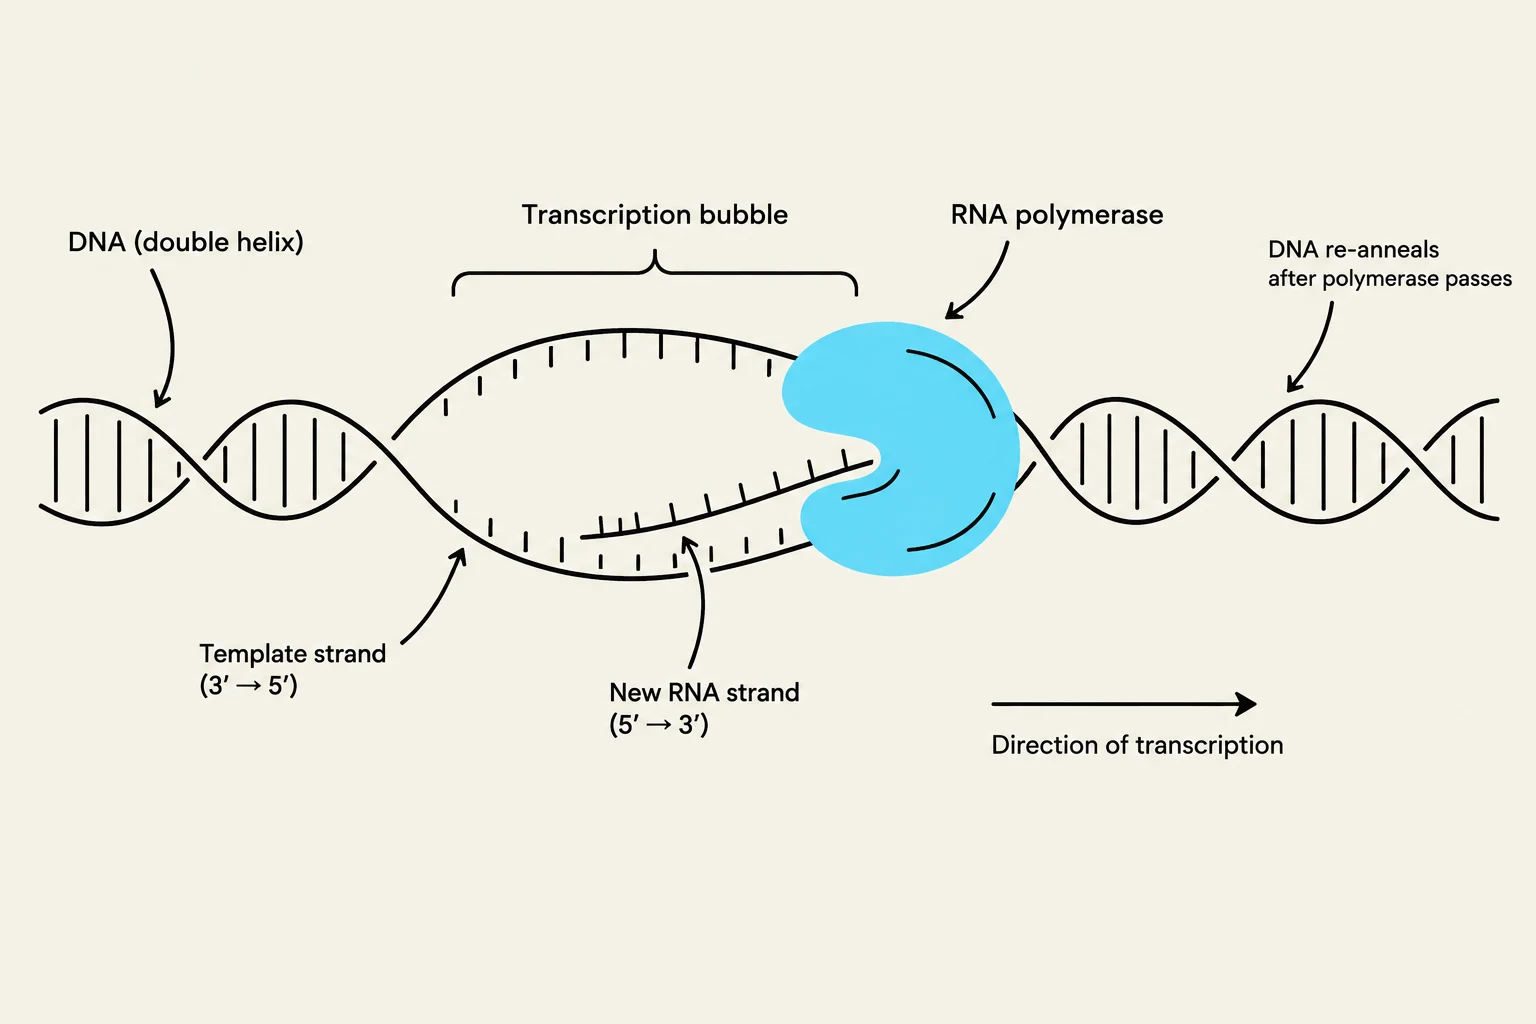
Open Complex: The polymerase undergoes a conformational change and unwinds the DNA to create a "transcription bubble," exposing the template strand.
Abortive Events: Before the enzyme can move into the elongation phase, it often undergoes "abortive initiation," where it produces small, incomplete RNA oligonucleotides.
Only after these abortive events and the subsequent release of the sigma factor can the polymerase transition into the elongation phase.
Elongation and Torsional Stress
During elongation, the RNA polymerase moves along the DNA template, synthesizing an RNA strand complementary to the DNA. As the enzyme progresses, it must unwind approximately 17 bp of DNA at a time.
This continuous unwinding and rewinding of the DNA helix generates significant torsional stress (supercoiling) ahead of and behind the polymerase. To prevent the DNA from becoming too tightly wound, which would stall transcription, the cell utilizes enzymes called topoisomerases to relieve this tension.
Furthermore, prokaryotes can adapt to environmental changes, such as heat shock, by utilizing different sigma factors that direct the RNA polymerase to different sets of promoters.
Diagram illustrating the process of transcription, where RNA polymerase synthesizes a new RNA strand using a DNA template.
Termination: Ending the Message
Transcription must be terminated precisely to ensure that only the intended RNA sequences are produced. Prokaryotes use two primary mechanisms to achieve this:
1. ρ-independent (Intrinsic) Termination
This mechanism relies on the DNA sequence itself. The transcribed RNA forms a stable hairpin structure (a loop) due to internal base pairing. This hairpin is immediately followed by a string of uracil (U) residues in the RNA that pair with adenine (A) residues in the DNA. Because the A-U hydrogen bond is relatively weak, the RNA-DNA hybrid is unstable, causing the RNA to dissociate from the template.
2. ρ-dependent Termination
This mechanism requires a specific protein called the ρ (rho) protein. The ρ protein binds to the growing RNA strand and "climbs" toward the $3'$ end. When the RNA polymerase encounters a specific DNA sequence that causes it to pause, the ρ protein catches up and facilitates the release of the mRNA from the DNA template.
Complex Regulation: The Lac Operon
In prokaryotes, genes involved in the same metabolic pathway are often clustered together into operons. These clusters are transcribed as a single, long mRNA molecule (polycistronic) under the control of a single promoter. The Lac operon in E. coli is the classic example, managing the metabolism of lactose.
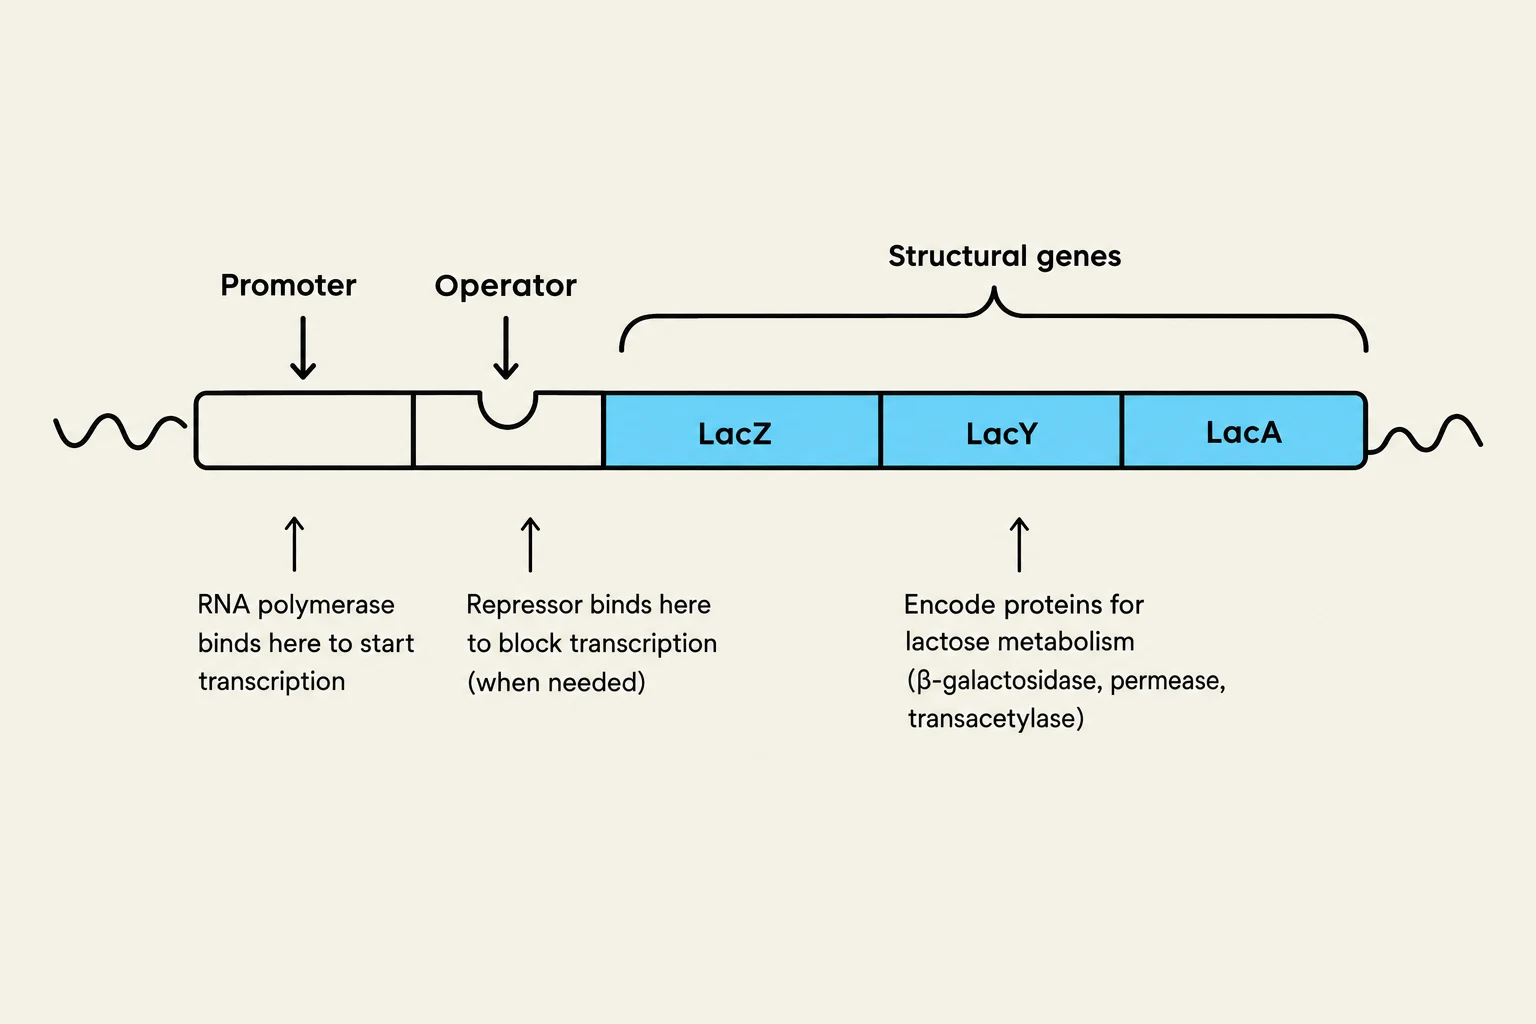
The Lac operon consists of three structural genes:
LacZ: Encodes β-galactosidase (breaks down lactose).
LacY: Encodes galactose permease (transports lactose into the cell).
LacA: Encodes thiogalactoside transacetylase.
Negative Regulation (The Brake)
The operon is subject to negative regulation by the Lac-repressor (encoded by gene I).
In the absence of lactose: The repressor binds to the operator sequence (O1), physically blocking RNA polymerase from transcribing the genes. This prevents the cell from wasting energy making enzymes it doesn't need.
In the presence of lactose: Lactose is converted into allolactose, which acts as an effector molecule. Allolactose binds to the repressor, changing its shape so it can no longer bind to the operator. This is called de-repression.
Positive Regulation (The Turbo-charger)
Even when lactose is present, E. coli prefers to use glucose because it is "easier" to metabolize. To ensure the Lac operon is only highly active when glucose is low, the cell uses positive regulation via the cAMP receptor protein (CRP).
Low Glucose → High cAMP: When glucose is scarce, levels of a signaling molecule called cAMP rise.
CRP Activation: cAMP binds to CRP, enabling CRP to bind to the CRP site on the DNA.
Transcription Boost: Once bound, CRP interacts with RNA polymerase, increasing its activity by approximately 50-fold.
Summary Table: The Lac Operon Logic
Glucose
Lactose
cAMP Level
CRP Bound?
Transcription Level
High
Absent
Low
No
Off (Repressed)
High
Present
Low
No
Low (Basal)
Low
Absent
High
Yes
Off (Repressed)
Low
Present
High
Yes
High (Induced)
Diagram illustrating the lac operon, showing the promoter, operator, and structural genes (LacZ, LacY, LacA) involved in lactose metabolism.
Through this dual-control system, the cell efficiently manages its resources, prioritizing the most energy-efficient fuel source available.
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.