Oxidative Phosphorylation and Mitochondrial Coupling
An in-depth explanation of oxidative phosphorylation, the electron transport chain, chemiosmotic coupling, and the roles of inhibitors and uncouplers in cellular energy production. It also covers reactive oxygen species and antioxidant defenses.
In the study of cellular metabolism, few processes are as fundamental as the production of energy via the mitochondria. While glycolysis provides a quick source of energy, it is significantly less efficient than the processes occurring within the mitochondria. To maximize ATP yield, cells utilize oxidative phosphorylation, a complex mechanism that integrates the movement of electrons with the synthesis of ATP. Understanding how these components are linked—and how that link can be broken—is essential for grasping both cellular bioenergetics and the mechanisms of various toxins and medications.
Oxidative Phosphorylation and the Electron Transport Chain
Oxidative phosphorylation is the process by which cells use enzymes to oxidize nutrients, thereby releasing energy which is used to reform ATP. This process is comprised of two highly interdependent stages: the Electron Transport Chain (ETC) and ATP synthesis.
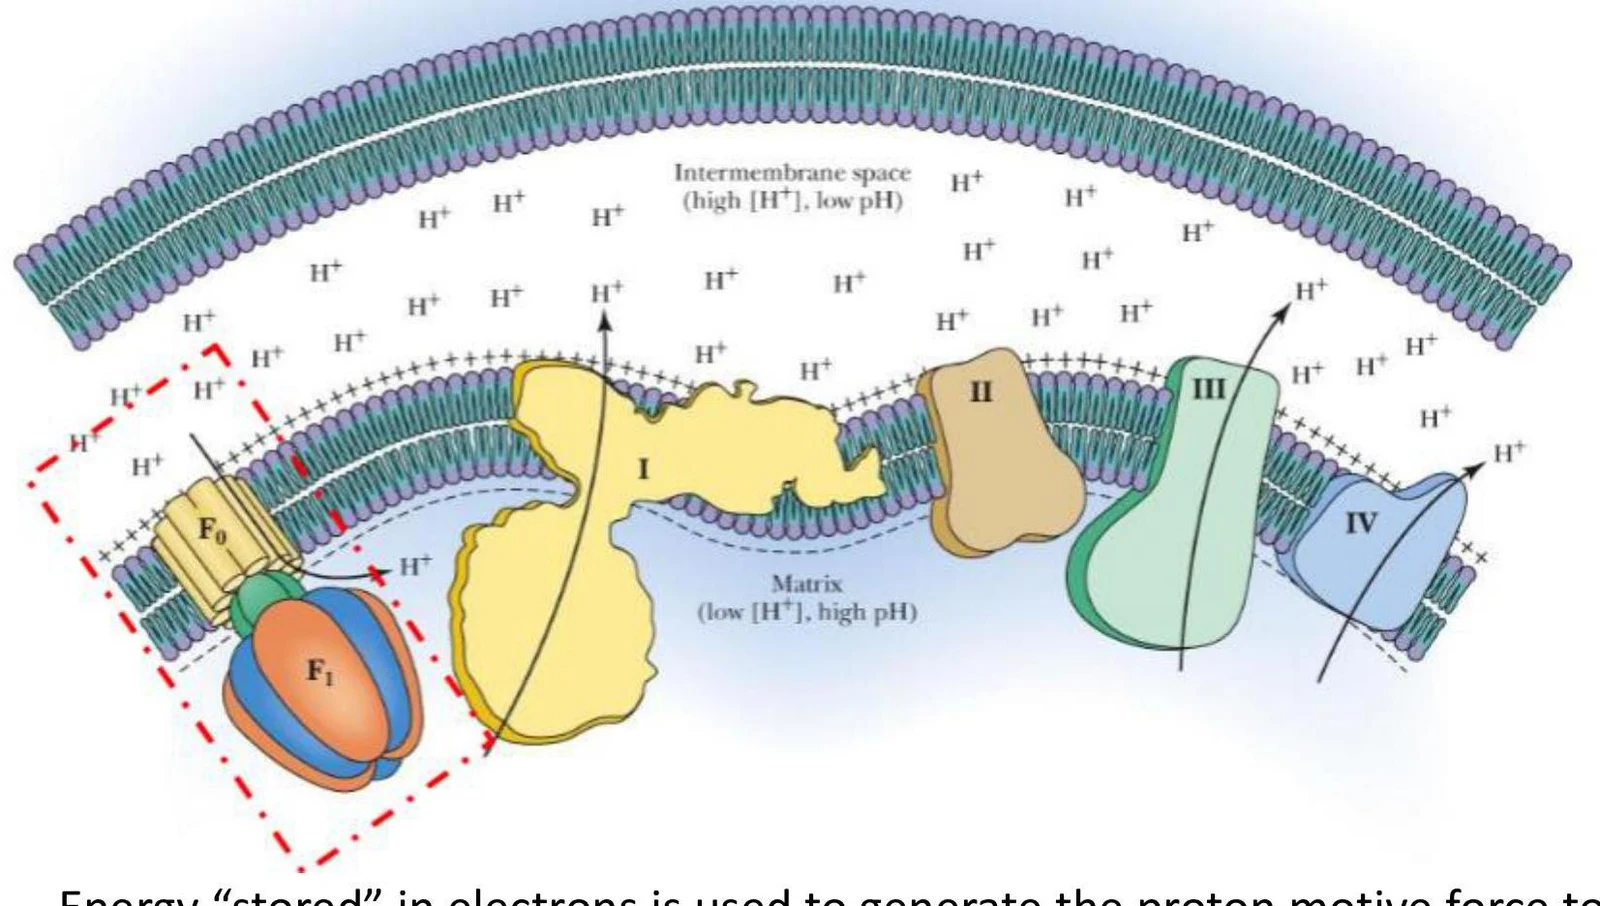
The Electron Transport Chain consists of a series of protein complexes embedded in the inner mitochondrial membrane. As electrons are passed from one complex to the next, energy is released. This energy is not lost as heat immediately; instead, it is used to pump protons ($H^+$) from the mitochondrial matrix into the intermembrane space. Oxygen (O2) plays a critical role here, acting as the final electron sink. Without oxygen to accept these electrons, the entire chain halts, preventing the formation of the proton gradient.
Diagram illustrating the electron transport chain and ATP synthase in cellular respiration, showing the movement of protons (H+) across the inner mitochondrial membrane to generate ATP.
Chemiosmotic Coupling and the Proton Motive Force
The link between the ETC and ATP synthesis is explained by the Mitchell Hypothesis, also known as Chemiosmotic Coupling. According to this theory, the energy stored in the electrons is used to establish an electrochemical gradient of protons across the inner membrane.
This gradient is known as the Proton Motive Force. The accumulation of protons in the intermembrane space creates both a concentration gradient and an electrical gradient. The only way for these protons to flow back into the mitochondrial matrix (down their gradient) is through a specialized protein complex called ATP synthase. As protons flow through ATP synthase, the mechanical energy of their movement is converted into chemical energy to drive the phosphorylation of ADP into ATP.
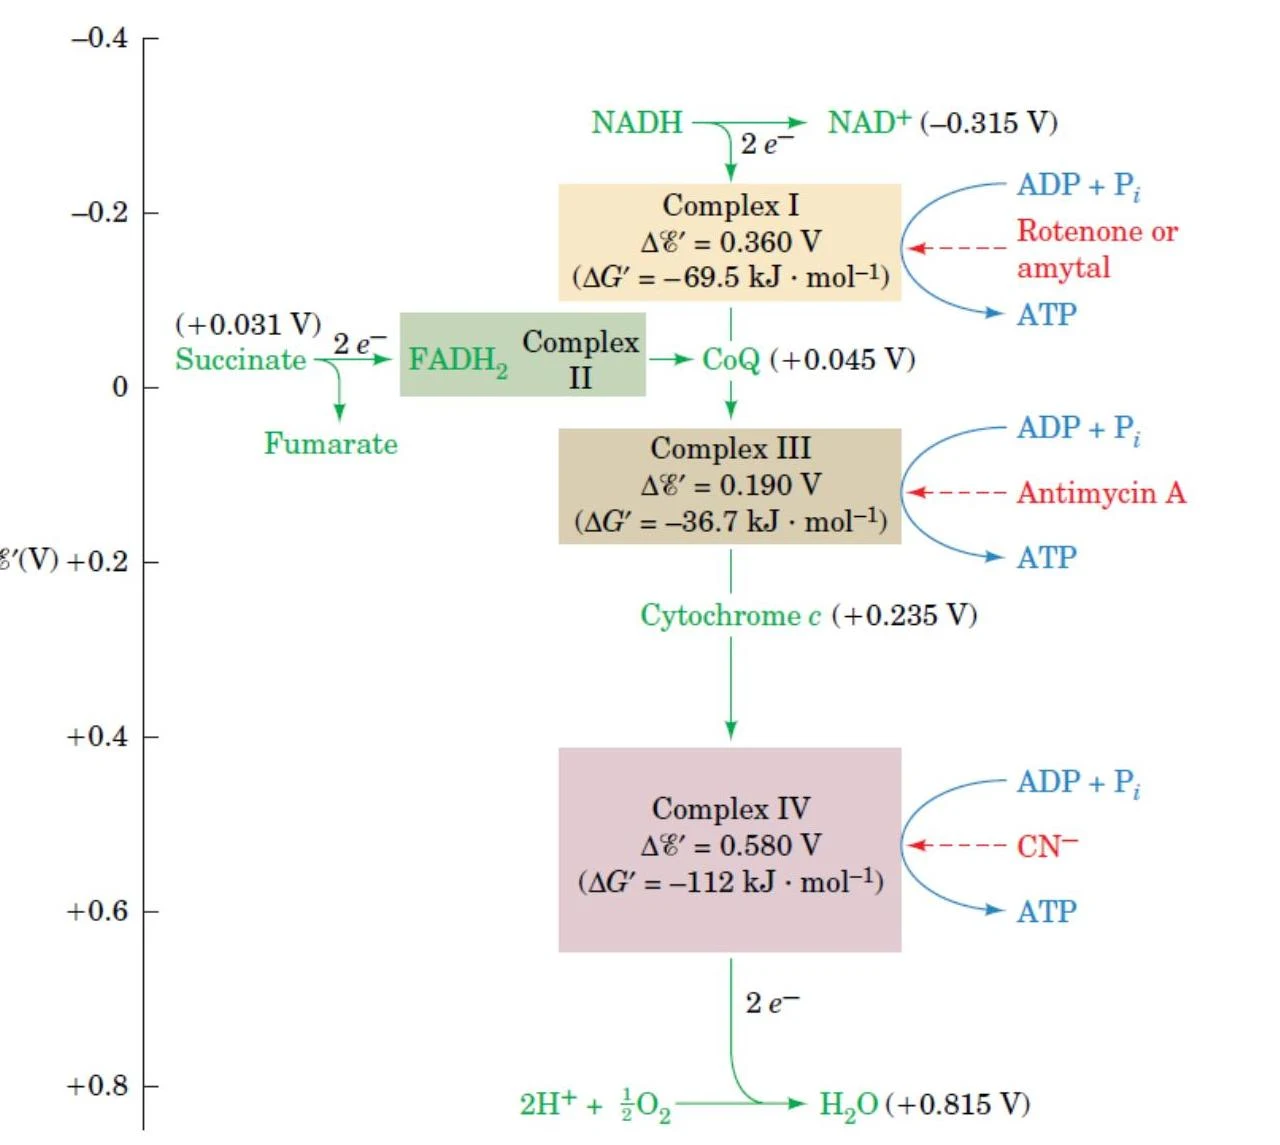
This diagram illustrates the electron transport chain, showing the complexes involved in cellular respiration, the associated changes in redox potential and free energy, and the production of ATP. Inhibitors like rotenone, antimycin A, and cyanide are also indicated.
Inhibitors of the Electron Transport Chain
Because the ETC is a sequential chain of redox reactions, inhibiting any single complex can halt the entire process of oxidative phosphorylation. Scientists use various inhibitors to study these pathways.
Complex I Inhibitors
Complex I is responsible for the initial oxidation of certain electron carriers. Rotenone is a naturally occurring inhibitor found in plant roots; it prevents the transfer of electrons from Fe-S clusters in Complex I to Coenzyme Q (CoQ). While used as a pesticide, it is also relevant in pharmacology. For example, certain medications like Demerol (an opioid analgesic) and Amytal (a barbiturate sedative) can act as CNS depressants and have been studied in the context of ETC inhibition.
Complex III Inhibitors
Antimycin A, produced by Streptomyces, inhibits Complex III by preventing electron flow from Cytochrome b to Coenzyme Q. A significant side effect of inhibiting Complex III is the increased production of Reactive Oxygen Species (ROS), which can be toxic to the cell.
Complex IV Inhibitors
Complex IV is the final step in the ETC before electrons are passed to oxygen. Inhibitors of this complex are often lethal. Cyanide is a classic example; it binds to the iron in heme a3 within Complex IV, preventing electron transfer. This causes an immediate halt in both oxygen consumption and ATP synthesis. Other notable inhibitors include Azide and Carbon Monoxide (CO).
Exam Tip: If you inhibit a complex in the ETC (like Complex IV with cyanide), both oxygen consumption and ATP synthesis will stop simultaneously. This demonstrates that the two processes are "obligately coupled".
ATP Synthase Inhibitors
While the previous inhibitors target the "engine" (the ETC), some substances target the "generator" (ATP synthase). Oligomycin A is a natural macrolide that binds to the F0 subunit of ATP synthase. By blocking the movement of protons through the F0 channel, it prevents the rotation required to synthesize ATP. Like cyanide, inhibiting ATP synthase will eventually cause oxygen consumption to slow down because the proton gradient becomes so steep that the ETC can no longer pump protons against it.
Uncouplers and Thermogenesis
What happens if we allow the protons to bypass ATP synthase? This is the role of Uncouplers. Uncouplers disrupt the tight link between the ETC and ATP synthesis by providing an alternative pathway for protons to leak back into the mitochondrial matrix.
When uncoupling occurs, the ETC continues to function (and often speeds up as it tries to restore the gradient), and oxygen is consumed, but the energy from the proton motive force is not captured as ATP. Instead, it is released as heat.
Chemical Uncouplers
Chemical uncouplers like FCCP or the infamous 2,4-Dinitrophenol (DNP) can diffuse across the mitochondrial membrane and carry protons directly into the matrix. DNP was once marketed as a weight-loss drug because it forces the body to burn fat to try and maintain ATP levels, but it was banned by the FDA in 1938 because it is highly unsafe and can be deadly.
Biological Uncouplers (Uncoupling Proteins)
Cells have evolved their own natural uncoupling proteins (UCPs) to manage energy and temperature:
UCP-1 (Thermogenin): Found in brown adipose tissue (BAT), it facilitates nonshivering thermogenesis by allowing protons to leak, generating heat to maintain body temperature in hibernating mammals or infants.
UCP-2 & UCP-3: Involved in protecting cells against the generation of Reactive Oxygen Species (ROS).
UCP-4 & UCP-5: Found primarily in the brain and testes.
Oxidative Stress and Antioxidant Defense
A major side effect of the ETC is the accidental production of Reactive Oxygen Species (ROS). When oxygen is partially reduced during electron transport, it can form superoxide (O2⋅−), the precursor to other highly reactive molecules. The most potent of these is the hydroxyl radical (⋅OH), which can be formed via Fenton Chemistry (the oxidation of hydrogen peroxide by iron).
Oxidative stress can damage vital biomolecules and lead to systemic issues in organs like the lungs, kidneys, and joints. To combat this, cells utilize an arsenal of antioxidants:
Superoxide Dismutase (SOD): The first line of defense, it converts superoxide into hydrogen peroxide (H2O2).
Glutathione Peroxidase (GPx): Uses the molecule glutathione (GSH) to reduce H2O2 into water (H2O). This process relies on the Pentose Phosphate Pathway (PPP) to provide the necessary NADPH to regenerate glutathione.
Catalase: An incredibly efficient enzyme that converts H2O2 into water and oxygen.
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.