Mechanisms of Transcription Elongation and DNA Supercoiling
Explores the intricate processes of transcription elongation, including navigating nucleosomal barriers and managing DNA supercoiling through topoisomerases.
Transcription is the fundamental process by which a cell interprets its genetic "history book" to produce functional messages. While initiation is the primary "on/off" switch for gene expression, the subsequent phase—transcription elongation—presents a formidable physical challenge. The RNA polymerase II (Pol II) complex must navigate a crowded nuclear environment, physically pushing through tightly packed chromatin while managing the intense mechanical tension generated by its own movement.
Navigating the Nucleosomal Barrier
In eukaryotes, DNA is not a naked string; it is organized into nucleosomes, where approximately 200 base pairs of DNA wrap around a histone octamer. For transcription to proceed, RNA polymerase II must traverse these structures, which act as physical roadblocks.
To facilitate passage, the nucleosome undergoes a controlled cycle of partial disassembly and reassembly. This process is not random; it is carefully managed by elongation factors that guide the reassembly of histones in the polymerase's wake. This precise recycling is crucial for maintaining epigenetic memory, ensuring that the chromatin state is preserved even after the transcriptional machinery has passed.
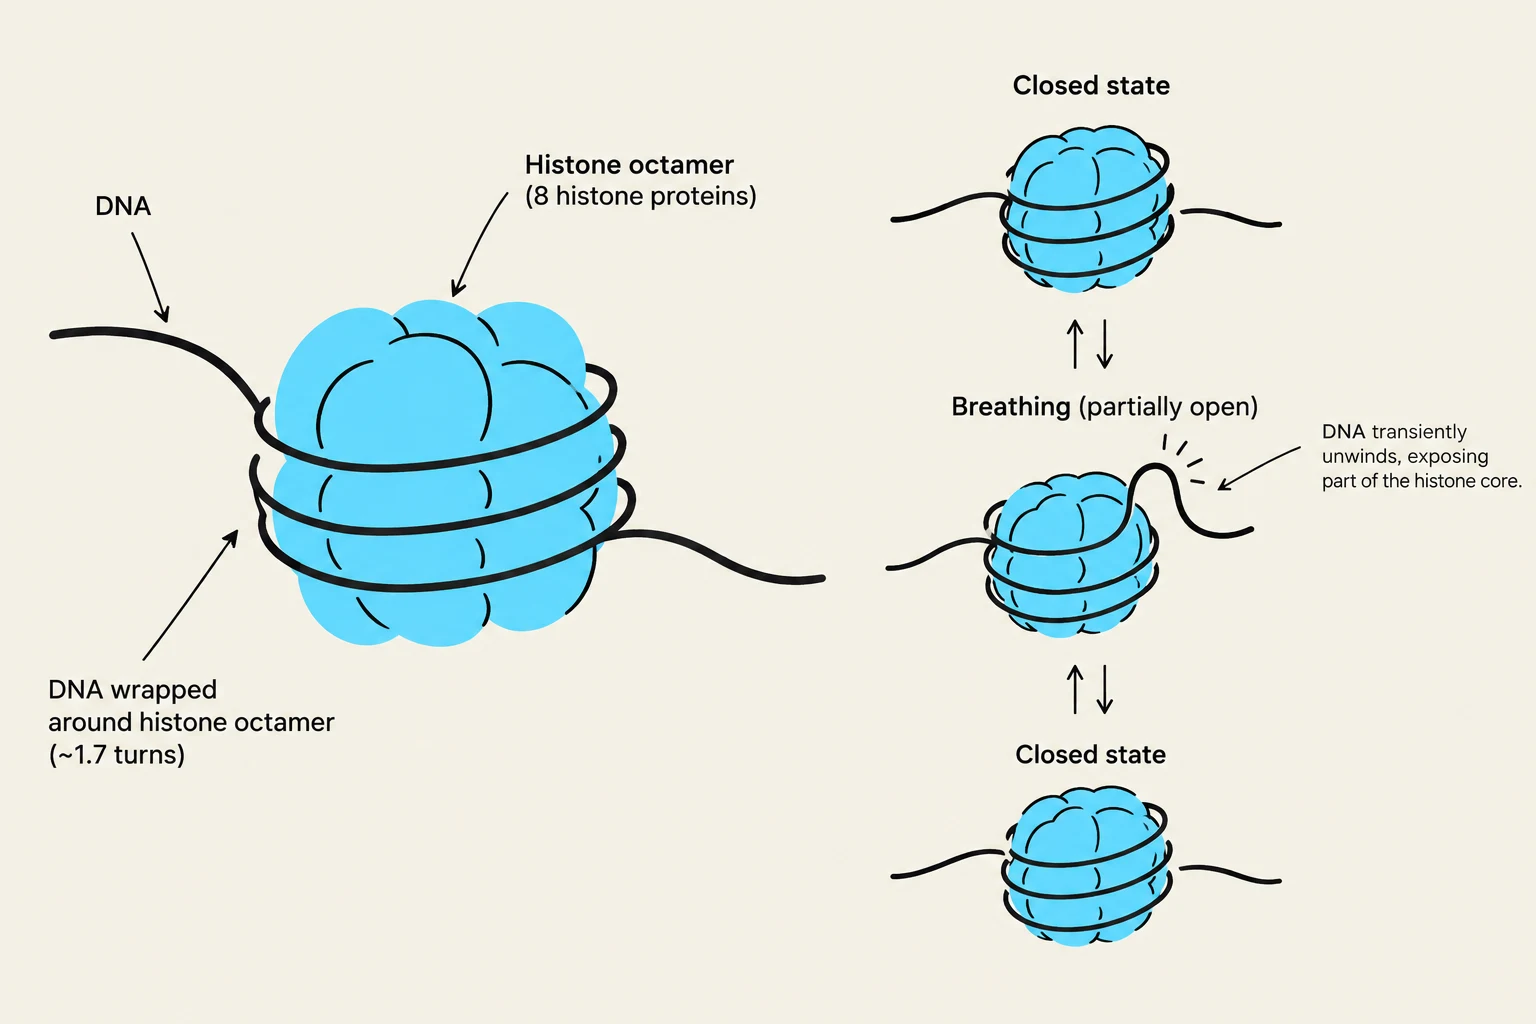
One way DNA interacts with histones is through a phenomenon called "breathing". This refers to the process where DNA transiently unwraps from the histone octamer, occurring roughly 5% of the time. Accessibility is not uniform: the affinity of DNA for the histone is significantly reduced at the ends of the nucleosome (by ~20x) and even more drastically at the middle (~200x).
Diagram illustrating DNA wrapping around a histone octamer and the dynamic process of DNA unwinding, referred to as breathing.
Chromatin Remodeling and Pioneer Factors
Because nucleosomes can block access to essential regulatory sequences, cells employ several mechanisms to manipulate chromatin structure:
Activators and HATs: Activators recruit Histone Acetyltransferases (HATs), which add acetyl groups to histones. These marks are then recognized by bromodomain readers within chromatin remodeling complexes.
Nucleosome Sliding: ATP-dependent remodelers use energy to slide nucleosomes along the DNA, exposing transcription factor (TF) binding sites and creating regions of nucleosome-free DNA.
Histone Variants: The incorporation of specialized histone variants can alter the stability of the nucleosome to allow greater accessibility.
Positive Feedback Loops: As TFs bind to newly exposed sites, they recruit more coactivators, which in turn drive further remodeling, creating a more favorable chromatin state for transcription.
A specialized class of proteins, known as Pioneer Factors, plays a critical role in initiating this process. Unlike standard TFs that require pre-existing nucleosome-free DNA, pioneer factors can bind to DNA even when it is still wrapped around a nucleosome. They achieve this by making simultaneous contact with both the DNA and the histone surface, partially destabilizing the nucleosome and subsequently recruiting ATP-dependent remodeling complexes to open the site for other factors.
Exam Tip: Remember that most TFs require "open" DNA, but Pioneer Factors are unique because they can "invade" closed chromatin to start the remodeling process.
The Dynamics of DNA Binding
How do transcription factors find their targets among 3 billion base pairs? Most TFs exist in a state of freely diffusing high mobility, performing a random 3D search through the nucleus at rates of approximately 1 µm2 per second. They sample thousands of sites per second, only pausing (low mobility) when they encounter a high-quality binding site.
This illustration depicts two states of transcription factors: freely diffusing within the nucleus with high mobility, and DNA-bound with lower, site-specific mobility.
Managing Torsional Stress: DNA Supercoiling
As RNA polymerase II moves along the DNA, it acts like a bulky machine moving through a twisted rope. Because chromosomes have fixed ends and the polymerase is too large to rotate freely around the DNA, the movement of the enzyme generates significant torsional tension known as DNA supercoiling.
This tension manifests in two distinct ways:
Positive Supercoiling: The DNA becomes overwound in front of the moving polymerase.
Negative Supercoiling: The DNA becomes underwound behind the polymerase.
If this tension is not relieved, the DNA becomes so tightly coiled that the polymerase can no longer progress, effectively halting transcription.
The Role of Topoisomerases
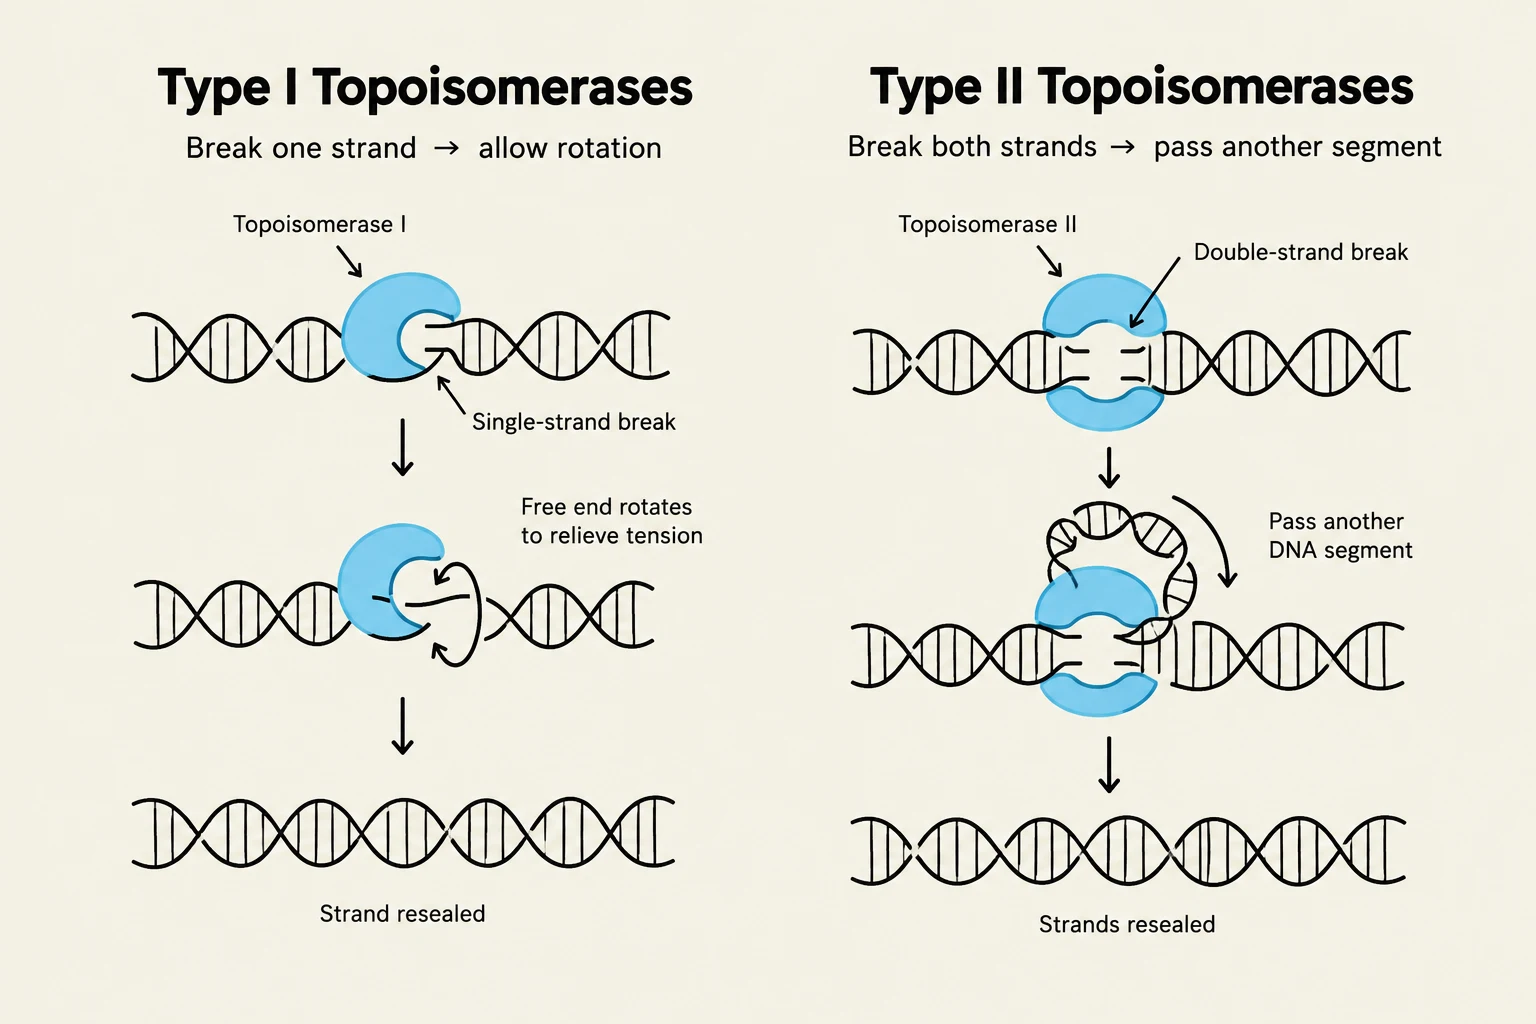
To prevent transcriptional arrest, cells utilize specialized enzymes called topoisomerases to relieve this torsional stress by temporarily breaking the DNA backbone. There are two primary classes:
Type I Topoisomerases: These enzymes break a single strand of the DNA duplex. This allows the DNA to rotate around the intact strand, relaxing one supercoil per cycle before the break is resealed.
Type II Topoisomerases: These are more efficient for high-tension scenarios. They break both strands of the DNA, allowing another segment of the DNA duplex to pass through the break before resealing it. This mechanism allows them to relax multiple supercoils more rapidly.
Diagrams illustrating the mechanisms of Type I and Type II topoisomerases in DNA manipulation.
Summary Table: Topoisomerase Comparison
Feature
Type I Topoisomerase
Type II Topoisomerase
Strands Broken
Single strand
Both strands
Mechanism
Rotation around intact strand
Passing a duplex through the break
Efficiency
Relaxes 1 supercoil per cycle
Relaxes multiple supercoils
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.