Explores the sophisticated mechanisms of eukaryotic gene regulation, focusing on histone modification and the GAL gene system in yeast for galactose metabolism. Details chromatin structure, acetylation, and the interplay of repressors and activators in response to nutrient availability.
In the complex world of eukaryotic cells, survival depends on the ability to sense the environment and adjust metabolic processes accordingly. One of the most elegant examples of this ability is found in yeast, which must decide whether to burn glucose—its preferred energy source—or switch to galactose when glucose is scarce. This decision is not merely a matter of turning a switch on or off; it involves a sophisticated dance of protein-DNA interactions, chromatin remodeling, and chemical modifications to histones that dictate whether a gene is accessible to the machinery of life.
The Fundamentals of Chromatin and Histone Modification
To understand how genes are regulated, we must first look at how DNA is packaged. In eukaryotes, DNA is not floating freely; it is wrapped around protein complexes called nucleosomes. Each nucleosome consists of eight core histone proteins (two each of H2A, H2B, H3, and H4).
The way these histones interact with DNA determines whether a gene is "open" for business or "locked" away. This interaction is primarily controlled through chemical modifications to the histone tails. By adding or removing specific chemical groups, the cell can alter the surface charge of the histone proteins, thereby changing their affinity for the negatively charged DNA.
Two primary types of modifications include:
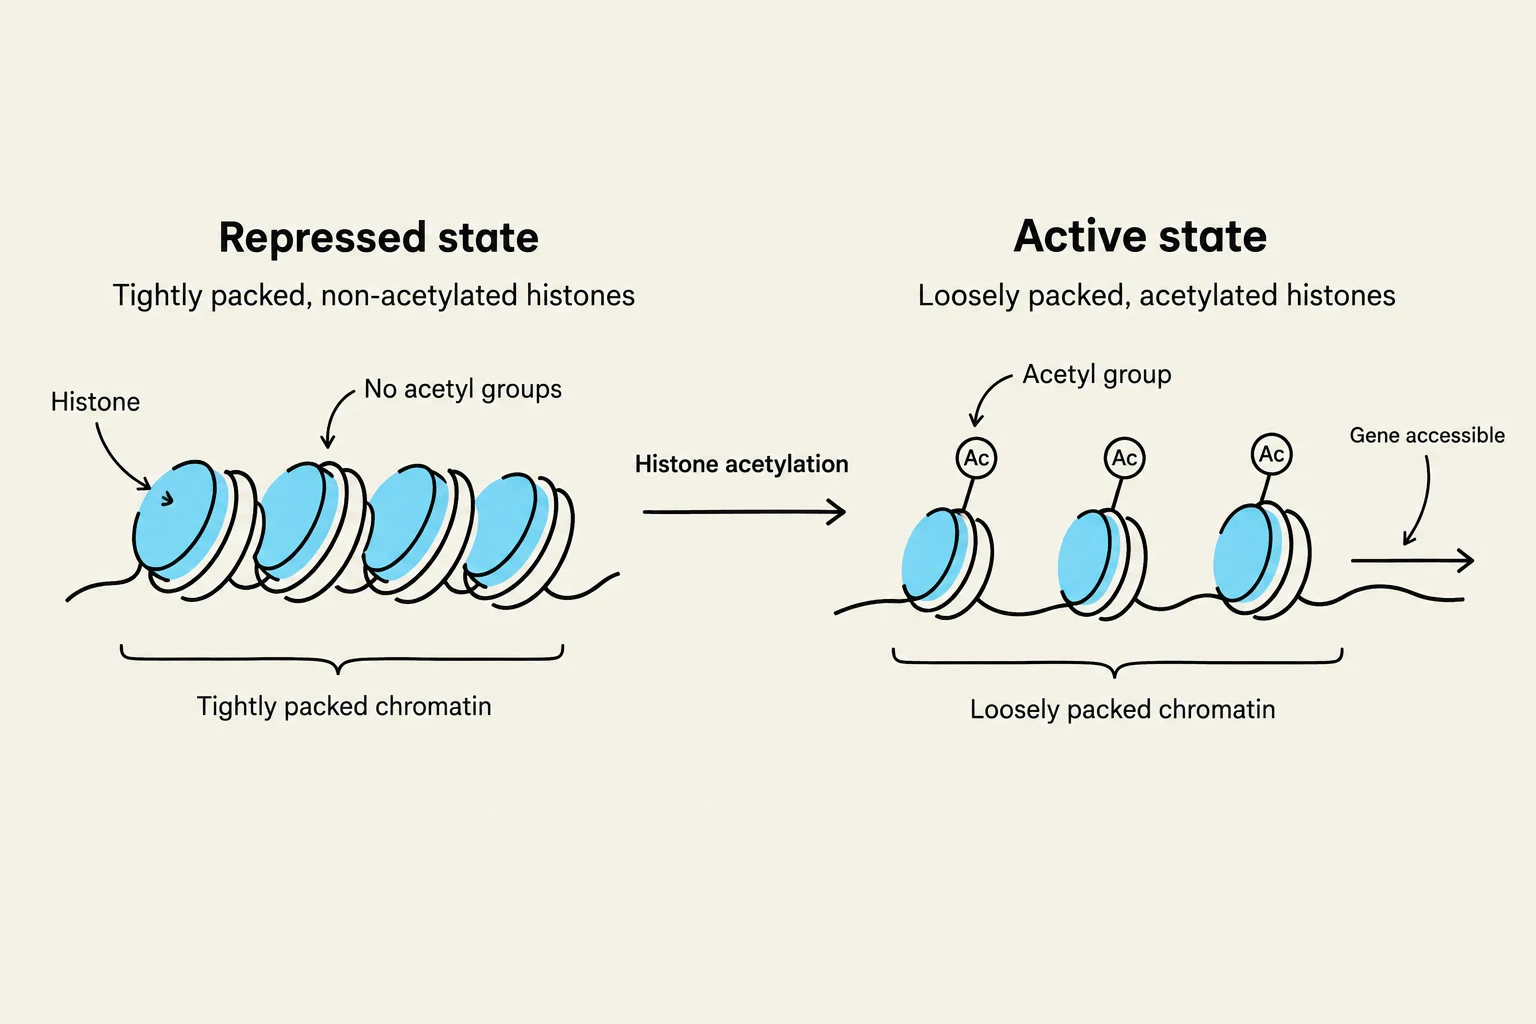
Acetylation: The addition of acetyl groups (−COCH3) to lysine amino acids via enzymes called Histone Acetyltransferases (HATs). Acetylation decreases the histone's grip on DNA, opening the chromatin structure.
Deacetylation: The removal of these groups, which causes the DNA to wrap more tightly around the histones, compacting the chromatin and silencing the gene.
Beyond acetylation, histones can also be modified via the addition of phosphate groups and methyl groups to further fine-tune the accessibility of the genetic code.
Diagram illustrating the difference between repressed and active chromatin states based on histone acetylation. In the repressed state, histones are tightly packed and non-acetylated, making genes inaccessible. In the active state, histone acetylation leads to loosely packed chromatin, allowing genes to be accessible.
Exam Tip: Remember the relationship between charge and structure. Acetylation neutralizes positive charges on histones, reducing their attraction to the negative DNA backbone, which leads to an "open" chromatin state.
The GAL Gene Family and Galactose Metabolism
In yeast, the ability to process galactose is governed by the GAL gene family, which includes three essential structural genes: $GAL1$, $GAL7$, and $GAL10$. These genes serve specific metabolic roles:
$GAL1$ (Galactokinase): Initiates the process.
$GAL7$ (Galactose transferase): Facilitates the transfer of sugar groups.
$GAL10$ (Galactose epimerase): Completes the conversion.
The ultimate goal of this pathway is to convert galactose into glucose-1-phosphate, a substrate that can enter the glycolysis pathway to produce energy. Because glucose is a more efficient energy source, the cell has evolved a strict regulatory hierarchy to ensure these GAL genes are only expressed when galactose is available and glucose is absent.
The Three States of GAL Regulation
The regulation of the GAL genes is highly sensitive to the available carbon source. The system operates in three distinct physiological states:
State
Carbon Source
Transcriptional Status
Inactive-Repressed
High Glucose
Genes are turned off; chromatin is compact.
Inactive-Poised
Glycerol
Genes are off, but ready for rapid induction.
Active-Induced
Galactose (No Glucose)
Genes are highly expressed.
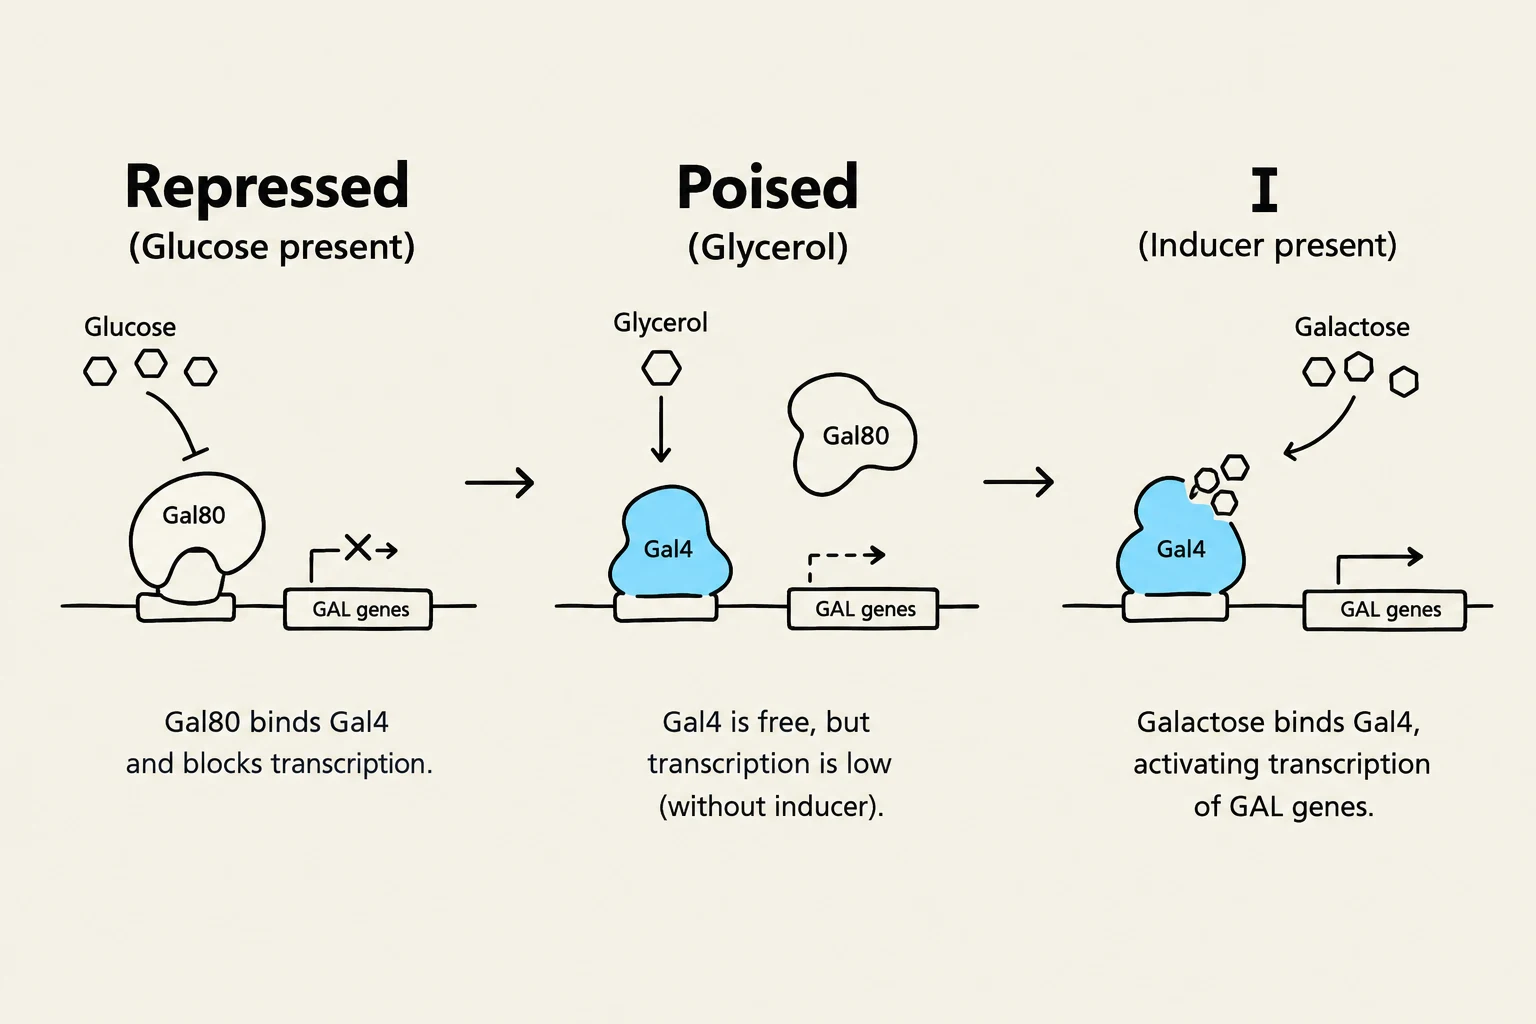
The master regulator of this system is the GAL4 protein, an activator that binds to a specific DNA sequence in the promoter called the Upstream Activator Sequence (UAS). Interestingly, GAL4 remains bound to the UAS regardless of whether galactose is present or not; the presence of galactose acts as the "key" that unlocks the ability of the bound GAL4 to initiate transcription.
This diagram illustrates the regulation of GAL genes in yeast. In the 'Repressed' state, glucose is present, and Gal80 binds to Gal4, blocking transcription. In the 'Poised' state, with glycerol present and no inducer, Gal4 is free but transcription is low. In the 'I' state, when an inducer (like galactose) is present, it binds to Gal4, activating the transcription of GAL genes.
Breaking the Repression: From Glucose to Galactose
When glucose levels are high, the cell must prevent the wasteful expression of GAL genes. This is achieved through a multi-layered repression mechanism involving the Mig1 repressor protein.
The Repression Mechanism (High Glucose)
Mig1 Binding: In the presence of glucose, the Mig1 protein binds to a specific site in the promoter near the UAS.
Tup1 Recruitment: Mig1 acts as a scaffold, recruiting the Tup1 co-repressor protein.
Chromatin Compaction: Tup1 then recruits Histone Deacetylase 1 (HDA1). HDA1 removes acetyl groups from the nearby histones, causing the DNA to wrap tightly and preventing the transcription machinery from accessing the genes.
The Induction Mechanism (Low Glucose + Galactose)
When glucose concentrations drop, the cell initiates a "relief" protocol to prepare for galactose metabolism:
SNF1 Activation: Low glucose triggers the activation of the SNF1 protein in the cytoplasm.
Nuclear Translocation: Once activated, SNF1 moves into the nucleus.
Phosphorylation and Removal: SNF1 phosphorylates both the Mig1 repressor and the co-activator Sip4. This phosphorylation causes Mig1 and its partner Tup1 to be released from the DNA.
Acetylation and Opening: With the repressors gone, the SAGA protein complex is recruited to the promoter. SAGA acts as a Histone Acetyltransferase (HAT), adding acetyl groups to the histones. This acetylation relaxes the chromatin, allowing RNA polymerase II and other transcription factors to bind and drive high-level expression of the GAL genes.
Through this sophisticated interplay of phosphorylation, acetylation, and protein recruitment, the yeast cell ensures that its metabolic machinery is perfectly tuned to its nutritional environment.
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.