ATP Synthesis and Chemiosmotic Coupling in Cellular Respiration
Explains the process of oxidative phosphorylation, where the electron transport chain creates a proton gradient (proton motive force) that drives ATP synthesis through ATP synthase, detailing the mechanisms of proton pumping, ATP synthase function, and the calculation of ATP yield from NADH and FADH2.
In the complex world of cellular respiration, the ultimate goal is the production of Adenosine Triphosphate (ATP), the universal energy currency of the cell. While the Electron Transport Chain (ETC) is responsible for moving electrons through various complexes, it does not produce ATP directly. Instead, it creates the necessary conditions for a remarkable molecular machine to do so. This process, known as oxidative phosphorylation, relies on the coupling of electron transport to ATP synthesis through a mechanism called chemiosmosis.
Chemiosmotic Coupling and the Proton Motive Force
The connection between the ETC and ATP synthesis is not a direct chemical reaction, but rather a coupling mediated by a proton gradient. As electrons flow through the respiratory complexes (Complexes I, III, and IV), protons ($H^+$) are actively pumped from the mitochondrial matrix across the inner mitochondrial membrane and into the intermembrane space.
Diagram illustrating the proton gradient across the inner mitochondrial membrane during cellular respiration.
This pumping creates a significant difference in proton concentration and electrical charge between the two sides of the membrane. This electrochemical gradient is known as the Proton Motive Force.
Thermodynamically, the protons "want" to flow back into the matrix to equalize the concentration and charge. The energy stored in this gradient is what drives the synthesis of ATP.
Diagram illustrating the electron transport chain and oxidative phosphorylation within the inner mitochondrial membrane, showing the movement of electrons through protein complexes and the pumping of protons (H+) to create a gradient that drives ATP synthesis.
The ATP Synthase Enzyme (F1/F0 ATPase)
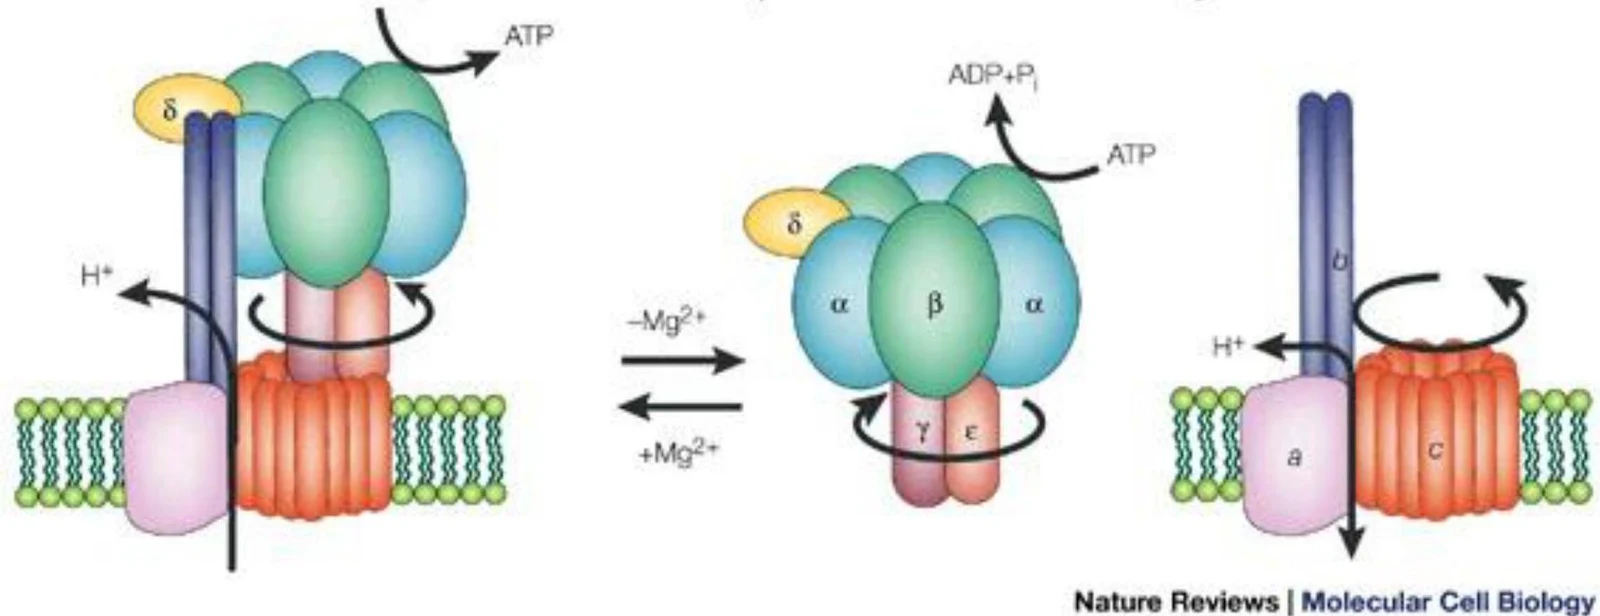
The cell harnesses the energy of the proton motive force using a specialized multimeric enzyme called ATP Synthase, also referred to as the F1/F0 ATPase. This enzyme acts like a molecular motor, converting the potential energy of the proton gradient into mechanical rotation, and finally into chemical energy stored in ATP.
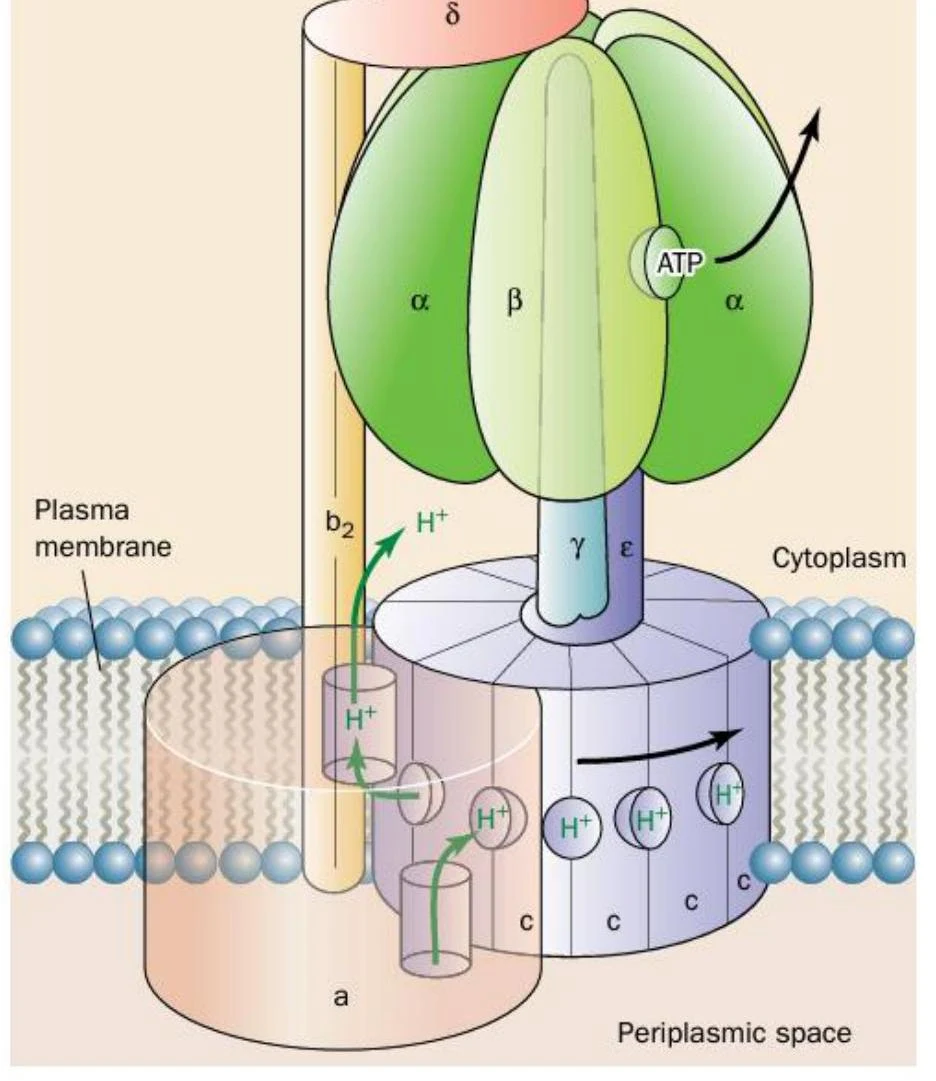
Diagram illustrating the mechanism of ATP synthase, showing the movement of protons (H+) across the plasma membrane to drive ATP synthesis in the cytoplasm.
The enzyme is composed of two distinct functional units:
The F0 Unit: This is the membrane-embedded portion of the enzyme. It acts as a rotor and provides the physical channel through which protons flow from the intermembrane space back into the matrix.
The F1 Unit: This unit is suspended in the mitochondrial matrix and is connected to the F0 unit by a central stalk subunit (the γ-stalk). The F1 unit is where the actual chemical synthesis of ATP occurs.
The F0 Rotor Mechanism
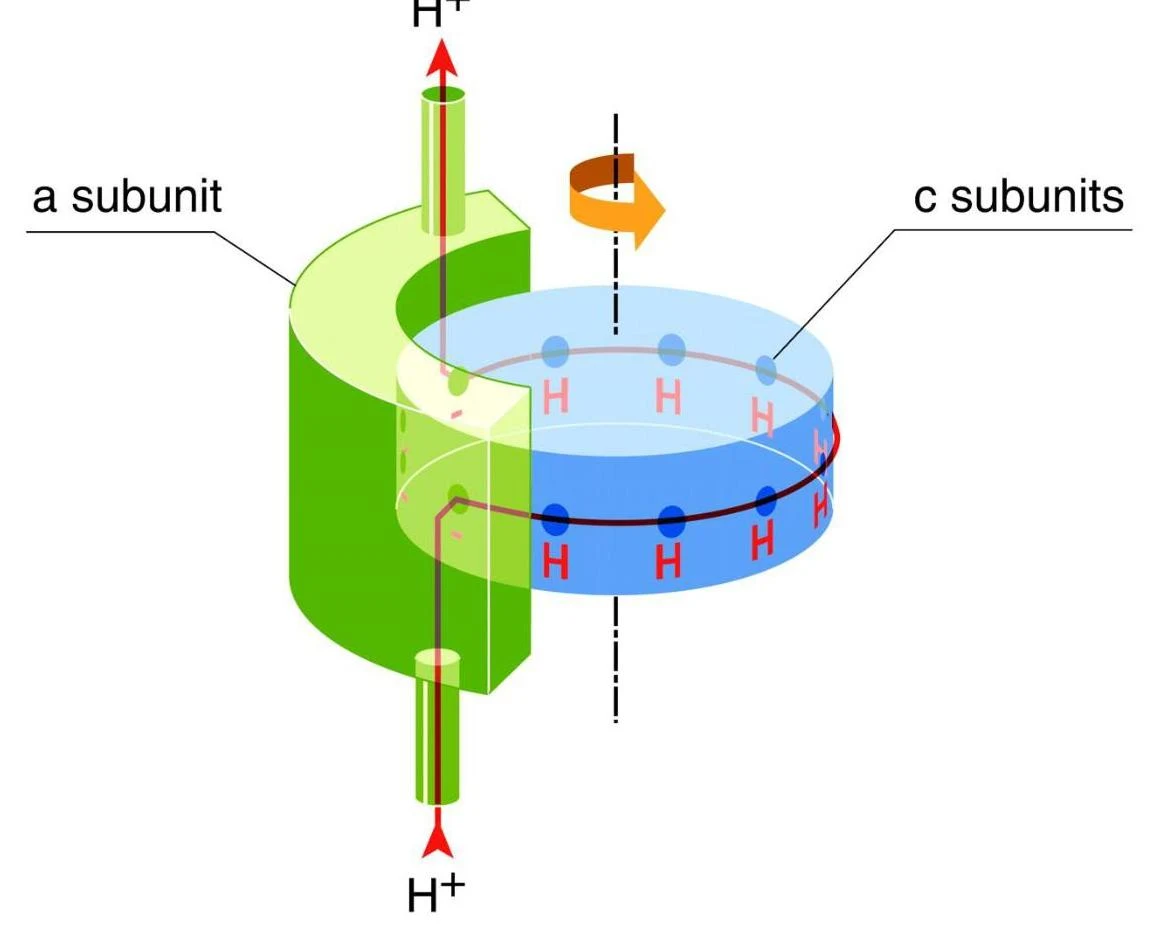
The rotation of the F0 unit is driven by the movement of protons through specific subunits. The F0 unit contains a subunits, which provide the passage for protons, and c subunits, which form the rotating ring.
As protons enter from the intermembrane space, they bind to glutamate or aspartate residues within the c subunits. This protonation causes the c subunit to lose its electrostatic interactions with a nearby arginine residue in the a subunit, which induces a clockwise rotation.
Diagram illustrating the function of the ATP synthase enzyme, showing the movement of protons (H+) through the c subunits and the rotation of the rotor.
The mechanics of this rotation are highly precise:
The movement of 3 $H^+$ induces a 120° turn of the rotor.
A full 360° rotation requires 9 $H^+$.
Rotational Catalysis in the F1 Unit
The mechanical energy from the F0 rotor is transmitted to the F1 unit via the γ-stalk. The F1 unit consists of three α (alpha) and β (beta) subunits arranged in a ring. While both subunits are present, the β subunits are the primary sites of catalysis.
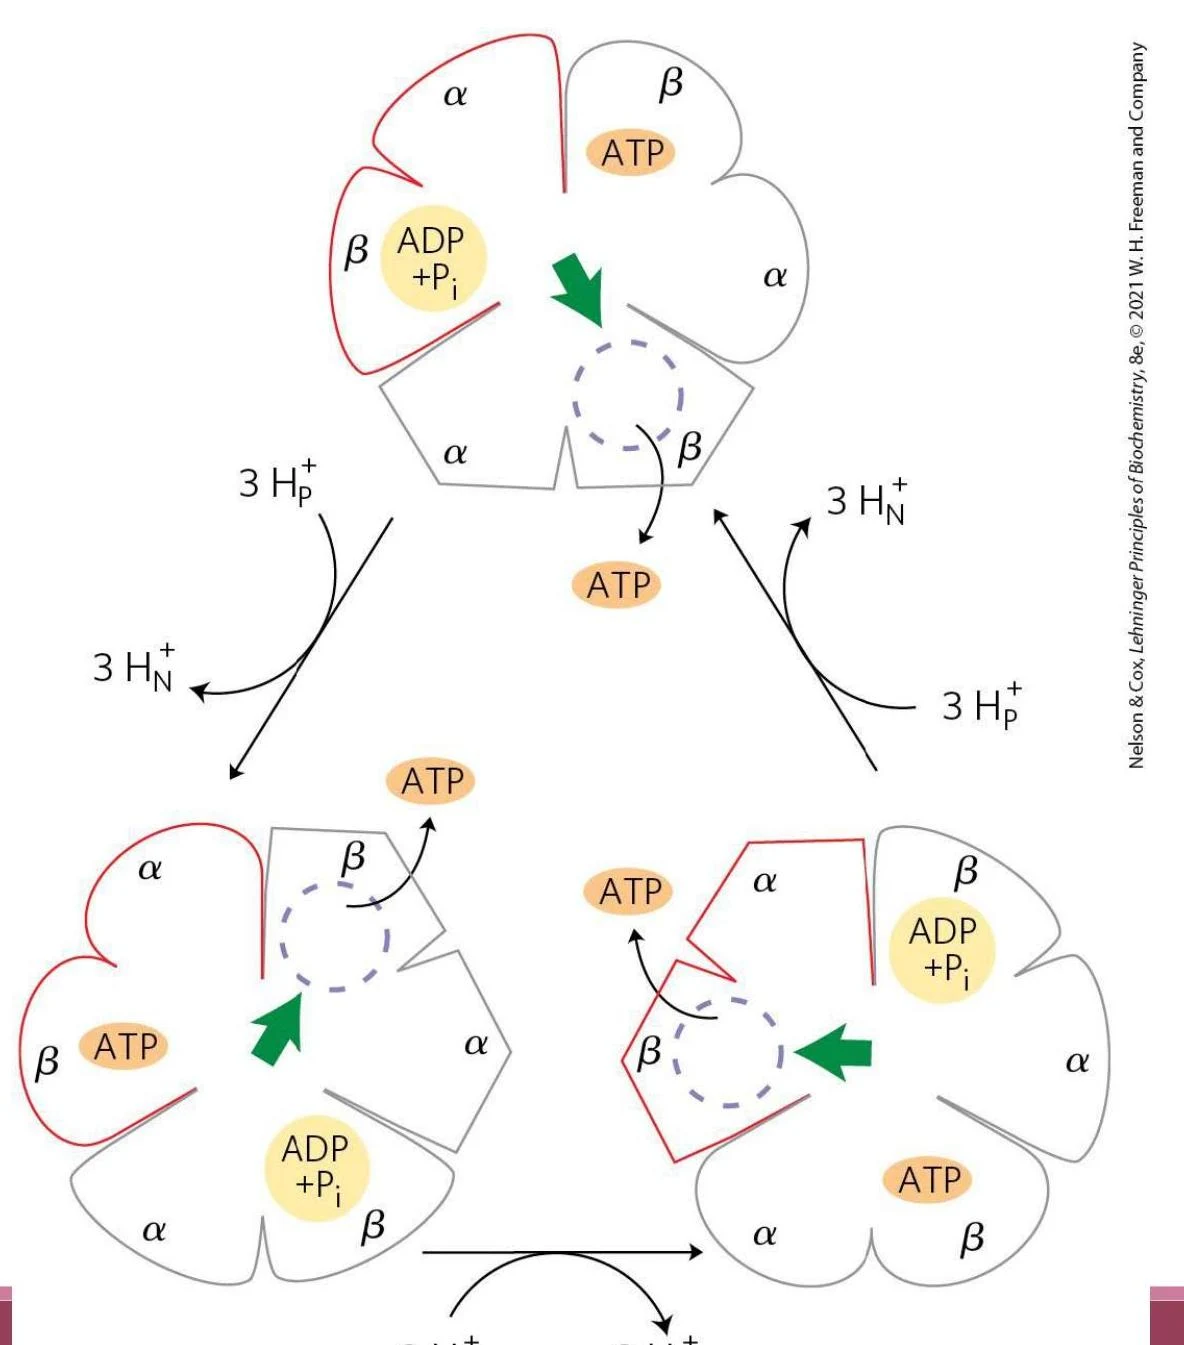
As the γ-stalk rotates inside the αβ ring, it forces the β subunits to undergo sequential conformational changes. This process is known as rotational catalysis.
Diagram illustrating the mechanism of ATP synthase, showing the rotation of subunits and the movement of protons and ATP.
At any given moment, the three β subunits are in different conformational states:
Open (O): The active site is empty and has a low affinity for substrates.
Loose (L): The active site is bound to ADP and inorganic phosphate (Pi), but they are not yet reacting.
Tight (T): The substrates are squeezed together so tightly that ATP is synthesized.
This diagram illustrates the mechanism of ATP synthase, showing the rotation of the gamma subunit within the alpha-beta subunits, driven by proton flow, to synthesize ATP from ADP and Pi.
Each 120° rotation of the stalk shifts each β subunit to the next conformation, resulting in the production of one ATP per subunit, for a total of 3 ATPs per full revolution.
The Energetics of ATP Production
To understand why this system is so efficient, we must look at the thermodynamics. The energy required to synthesize ATP in the mitochondria is approximately ΔG∘≈55–60 kJ/mol. In contrast, the energy provided by the flow of protons (the proton motive force) is roughly −21.5 kJ/mol per mole of protons.
ΔGA=RTlnΔpH+ZAFΔφ=−21.5 kJ/mol
Because the energy required for one ATP is greater than the energy provided by a single proton, it takes multiple protons to drive the synthesis of one ATP molecule. Specifically, based on the rotation of the enzyme, 3 $H^+$ are required to produce 1 ATP.
Exam Tip: Remember the distinction between the rotation of the enzyme and the total proton cost. While the F1 mechanism suggests 3 $H^+$ per ATP, you must account for the transport of molecules to get the "true" biological yield.
The Role of ATP-ADP Translocase
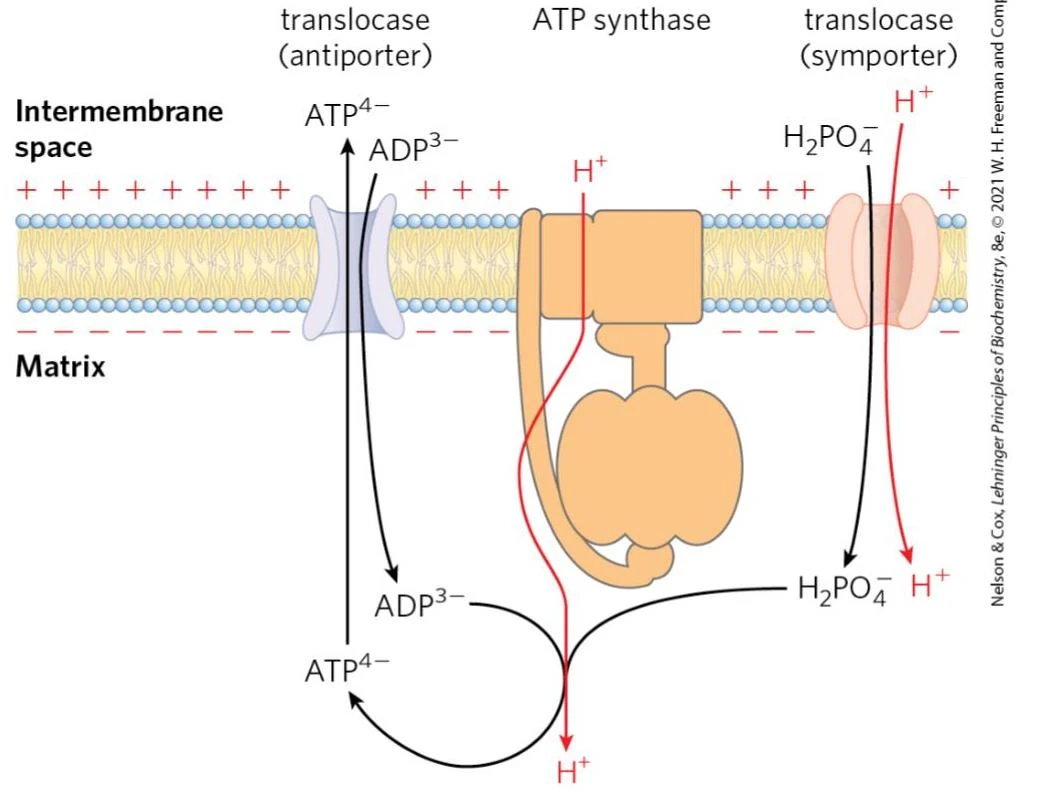
The ATP produced in the matrix must be exported to the rest of the cell, and the starting materials (ADP and Pi) must be imported. This is handled by the ATP-ADP Translocase.
ATP Export: ATP is exported out of the matrix in exchange for ADP. Since ATP is negatively charged, this exchange is energetically demanding.
Phosphate Import: Inorganic phosphate (Pi) is imported into the matrix via a symporter that also brings in 1 $H^+$.
When you combine the 3 $H^+$ needed for the rotation of ATP synthase with the 1 $H^+$ needed for phosphate transport, the total cost to produce and export one usable ATP molecule is 4 $H^+$.
Calculating ATP Yield
By knowing the total number of protons pumped by the ETC and the cost of 4 $H^+$ per ATP, we can calculate the ATP yield from different electron carriers.
From NADH:
NADH contributes 10 $H^+$ to the proton motive force via the ETC.
Yield: 4H+/ATP10H+=2.5 ATP.
From FADH2:
FADH2 contributes 6 $H^+$ to the proton motive force.
Yield: 4H+/ATP6H+=1.5 ATP.
This diagram illustrates the process of ATP synthesis in mitochondria, showing the roles of ATP synthase, a proton gradient, and various translocases in moving ions and molecules across the inner mitochondrial membrane.
Summary Table: Proton Cost and ATP Yield
Electron Carrier
Protons Pumped ($H^+$)
ATP Yield (at 4 $H^+$/ATP)
NADH
10
2.5
FADH2
6
1.5
(Note: Calculations assume the mitochondrial transport costs are included).
Keep reading for free.
Create an account to finish this reading and make it part of your study routine.